Key Points:
- Most of the nitrogen in a soybean seed is recycled from the leaves and stems, which is why fields yellow from the bottom up as pods fill.
- Nitrogen, phosphorus, and potassium remobilize efficiently while sulfur remobilizes on a separate timetable, and micronutrients like calcium don’t remobilize much at all.
- Late-season stress (heat, drought, defoliation, disease) can disrupt the remobilization process.
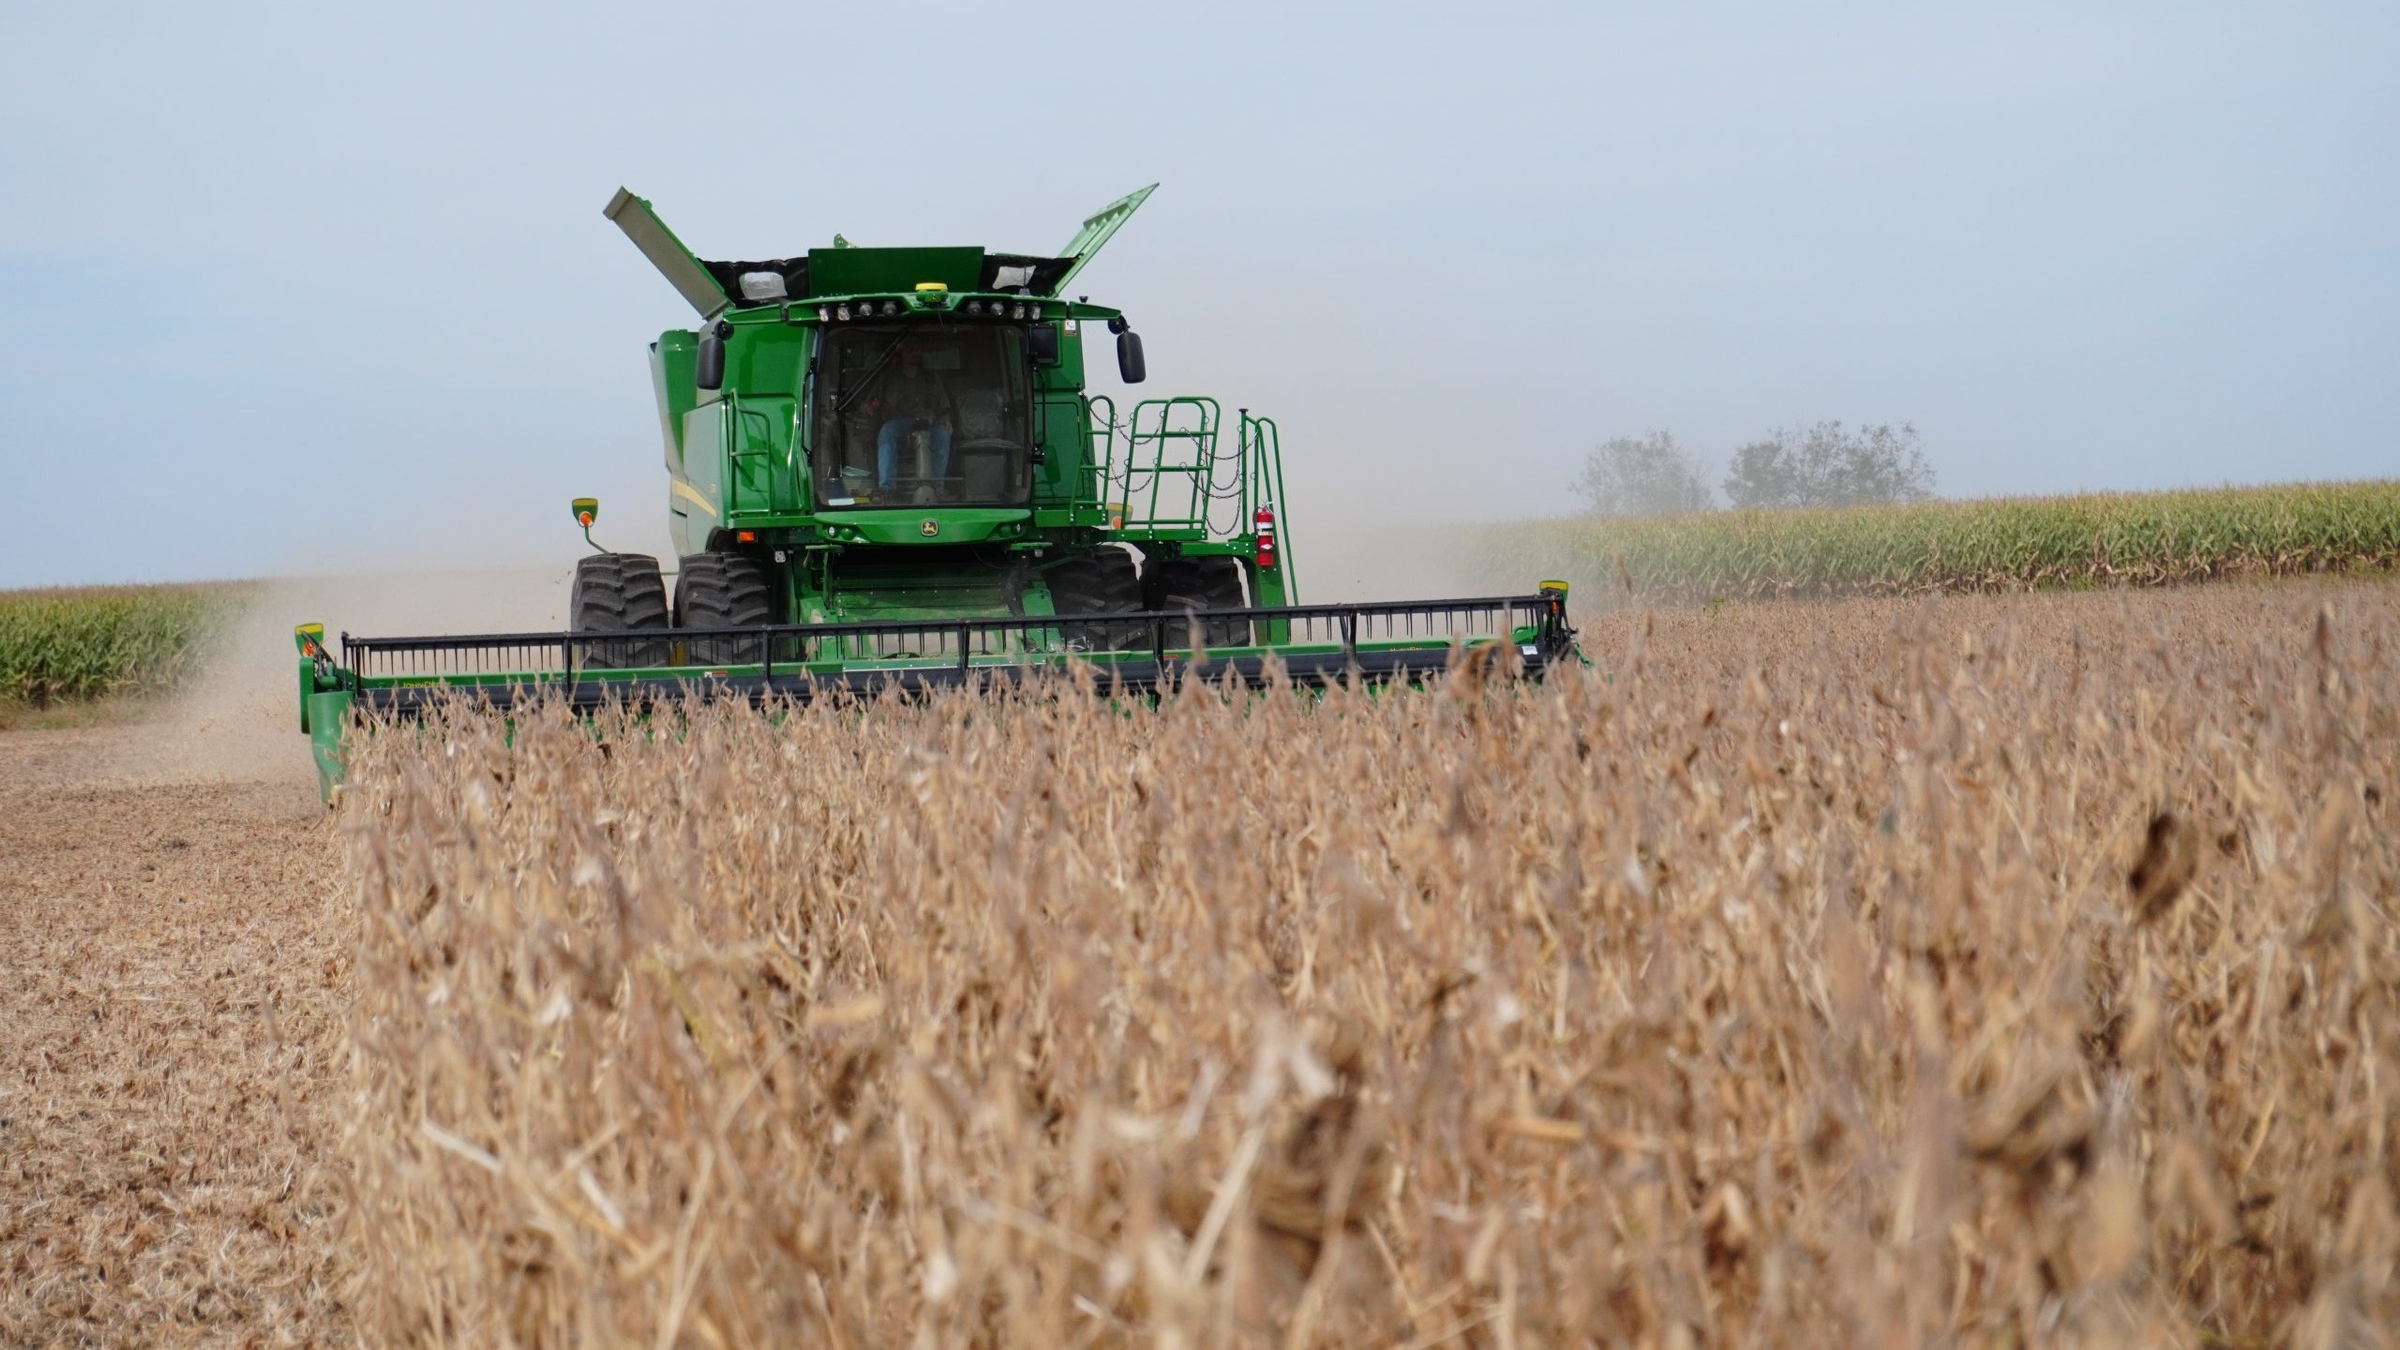
If you’ve ever watched a soybean field turn gold from the bottom up in late August, you’ve watched nutrient remobilization happen in real time. The plant dismantles its own leaves to feed the seeds above. Proteins in the plant and seed require significant energy and nitrogen for their synthesis. Much of the protein in a soybean seed comes from nutrients that were invested in the leaves and stems months earlier. This movement explains why fields senesce the way they do, why extra nitrogen fertilizer often fails to pay, and why late-season stress can quietly cap yield and protein.
What Is Nutrient Remobilization?
Nutrient remobilization is the movement of nutrients out of vegetative tissue like leaves, stems, and petioles into developing seeds, distinct from direct uptake by roots from the soil. Both happen during seed fill, but soybean leans unusually hard on remobilization, especially for nitrogen. Although it’s called an oilseed, soybean behaves like a protein storing legume. Soybean seed contains around 35% protein1 or 1260 lbs. of protein from a 60 bushel per acre crop. This equates to around 200 lbs. of N per acre. This is more nitrogen than the plant can typically acquire from the soil and biological fixation alone during the short seed-fill window. So, it taps reserves built earlier. An estimated 59% of seed nitrogen is derived from remobilization of vegetative nitrogen accumulated from soil uptake and biological fixation earlier in the season2, with older estimates ranging from 30% to 100% depending on genotype.3 Seed fill is fundamentally a recycling operation.
Which Nutrients Move and Where?
Nitrogen is stored in leaves largely in functional photosynthetic proteins such as Rubisco, as those break down during senescence. Amino acids move through the phloem to the seed and are the main drivers of late-season leaf yellowing. Stems matter too – soybean stems accumulate nitrogen through vegetative storage proteins that are later mobilized to support seed fill in high-yielding crops.4 Remobilization of functional biological machinery creates a self-destruction of the plant that terminates plant growth and initiates maturity.
Phosphorus and potassium also remobilize, but phosphorus doesn’t appear to drive senescence timing itself. Research across deficient, optimum, and excess soil phosphorus found that leaf senescence patterns were similar across all treatments, suggesting phosphorus nutrition doesn’t exert regulatory control over the process.5
Sulfur, needed for seed protein synthesis, runs on its own schedule and is generally considered independent of senescence.6 Expanding soybean leaves seem to better utilize newly acquired sulfur than mobilized forms; however, pods and seeds are better able to utilize remobilized sulfur.7 Pods are especially important for obtaining remobilized sulfur from vegetative tissues to support seed sulfur needs.
Micronutrients move the least. Calcium and manganese show essentially no apparent remobilization and accumulate in leaves even during senescence.6
Remobilization Timing
While nutrient mobilization from lower, shaded leaves may begin as early as R4; new leaves may be added until about midway between R5 and R6 when seed growth hasn’t yet taken off. Early nutrient mobilization is likely occurring from older to younger leaves. Remobilization ramps up from the beginning seed (R5) through beginning maturity (R7) stages. At R5, the plant is less able to compensate for stress. It redistributes stored nutrients to supply about half of its nitrogen, potassium, and phosphorus needs, with the rest coming from soil uptake and biological fixation and root uptake.8 By R5.5, the plant isn’t as able to compensate for stress and relies heavily on stored nutrients to meet a large share of its nitrogen, potassium, and phosphorus needs. Pod weight peaks and lower leaves naturally begin to yellow by R6, with senescence speeding up or slowing down depending on weather.8 R7 is the cutoff time. Seed fill stops once a pod loses its green color.9 Heat, drought, disease, or defoliation can accelerate senescence, reducing seed protein, seed size, and yield.

Remobilization Impacts on Yield and Quality
Yield and seed composition are tightly interconnected. Because protein and oil make up more than 60% of the seeds’ dry weight, biological drivers of protein and oil accumulation in the seed affect both quality and quantity of seed. And because seed protein is so highly dependent on nitrogen remobilization, anything that changes stored nitrogen or how efficiently it moves shows up in seed composition. Increasing nitrogen uptake, storage, and later remobilization coupled with increased late-season nitrogen accrual leads to higher yields and increased seed protein concentration.10 On the other hand, increased stay-green through delayed senescence can increase carbon allocation to the seed increasing both yield and oil content.10,11
Management Implications
Late-season nitrogen applications rarely deliver reliable payoffs. Across more than 200 U.S. environments, nitrogen fertilization has produced mixed and unreliable results.12 Responses cluster mainly in irrigated, high-yielding fields above roughly 60 to 65 bushels per acre with low soil organic matter and low available nitrogen.13 One study found significant yield gains at six of eight irrigated sites, averaging about 7 bushels per acre while non-responsive sites were simply lower-yielding.14
Managing stress from R4 to R7 is critical. Cerrudo and Naeve (2025) found that reduced carbon availability due to general stress has its greatest impact in the R5-R6 stages.15 However, follow-up work found generalized stress to impact both protein and oil accumulation similarly.16 On the other hand, defoliation during this period reduces both carbon and nitrogen availability, leading to reduced yield and seed protein content.
Variety selection is also worth discussing. Todeschini et al. (2019) and others have found that modern varieties are better at remobilizing nutrients primarily through increased harvest index.17 More practically, soybean maturity can affect both the quantity of stored minerals and remobilization efficiency. Shorter-than adapted varieties tend to have limited vegetative biomass and therefore are limited in the quantity of mobilizable nutrients. On the other hand, longer-than adapted varieties may run out of time to efficiently remobilize nutrients before frost or freeze events in the fall.
Conclusion
Soybean seed protein depends heavily on nutrients recycled from the plant’s own leaves and stems, not just new nutrient uptake from soil or biological fixation. Nitrogen, phosphorus, and potassium remobilize efficiently and largely follow the senescence process while sulfur moves on a separate timeline. Micronutrients like calcium barely remobilize at all. Remobilization is concentrated in the R5-R7 window and stress during this period can shorten it, capping both yield and seed protein. Late-season nitrogen applications are not a reliable fix for remobilization limits in typical rainfed fields. Protecting canopy health and choosing well-adapted varieties matter more.
Authors
Sagnika Das, University of Illinois Urbana-Champaign and Seth Naeve, University of Minnesota
Published October 21, 2026